Abstract
Objective: To establish a rapid TaqMan probe-based qPCR assay for genotyping the GLP1R rs6923761 polymorphism and to determine its concordance with Sanger sequencing.
Methods: Genomic DNA was isolated from buccal swabs collected from 22 adolescent volunteers. Each sample was genotyped by TaqMan qPCR and Sanger sequencing. DNA concentration and purity were assessed before amplification. Genotype and allele frequencies, Hardy-Weinberg equilibrium (HWE), overall concordance, Cohen’s kappa, and the exact 95% confidence interval (CI) for concordance were calculated.
Results: TaqMan qPCR identified 11 GG and 11 GA samples; no AA homozygote was observed. The G and A allele frequencies were 75.0% and 25.0%, respectively. Sanger sequencing gave identical genotype calls for all 22 samples. Concordance was 100% (22/22; exact 95% CI, 84.6%-100%), with a Cohen’s kappa of 1.00. Genotype distribution did not deviate significantly from HWE (chi-square = 2.44, p = 0.118).
Conclusions: In this initial sample set, the TaqMan qPCR assay distinguished the GG and GA genotypes of GLP1R rs6923761 with complete concordance to Sanger sequencing. The closed-tube workflow is suitable for further evaluation as a rapid assay for known-SNP genotyping. Because AA samples were unavailable and analytical sensitivity and reproducibility were not formally tested, additional validation is required before clinical or pharmacogenetic use.
Keywords: GLP1R; rs6923761; TaqMan qPCR; Sanger sequencing; SNP genotyping
Introduction
Overweight and obesity are increasingly common among children and adolescents in China, accompanied by a rising burden of metabolic disease and early-onset type 2 diabetes1,2,3. Lifestyle, nutrition, and physical activity remain major determinants, but genetic variation may also contribute to differences in metabolic traits and in response to incretin-based therapies4,5,6.
The glucagon-like peptide-1 receptor gene (GLP1R) encodes the GLP-1 receptor (GLP-1R), a 463-amino-acid class B G-protein-coupled receptor7. rs6923761 is a common missense variant in GLP1R in which a G>A substitution results in p.Gly168Ser8,9. The variant has been examined in relation to endogenous GLP-1 responses, insulin secretion, gastric emptying, obesity-related traits, type 2 diabetes, gestational diabetes, and response to GLP-1 receptor agonists (GLP-1RAs)8,9,10,11,12,13,14. The clinical significance of rs6923761 remains unsettled. Several small studies have reported associations with metabolic traits or responses to liraglutide and exenatide, including gastric emptying and glycemic outcomes, whereas larger pharmacogenomic analyses suggest that treatment effects may vary across phenotypes and populations10,11,12,13,14.
At present, rs6923761 is better considered a candidate pharmacogenetic marker than a validated predictor of GLP-1RA efficacy, weight loss, glycemic response, or dose.
Sanger sequencing provides direct sequence confirmation but requires PCR product processing and is relatively labor-intensive when large numbers of samples are tested. TaqMan allelic discrimination uses allele-specific fluorescent probes in a closed-tube PCR format and is well suited to rapid genotyping of known SNPs15,16,17,18,19.
| Feature | Sanger Sequencing | TaqMan-qPCR SNP Genotyping |
| Principle | Chain-termination sequencing; reads the target sequence | Allele-specific fluorescent probe hybridization and cleavage |
| Throughput per run | Typically, 24-96 samples | Typically, 96-384 samples |
| Turnaround time | Approximately 8-24 hours depending on workflow | Approximately 1.5-3 hours depending on workflow |
| Cost per sample | Relatively high | Relatively low after assay setup |
| Contamination risk | Higher due to multiple open-tube steps | Lower due to closed-tube amplification and detection |
| Key characteristic | Sequence confirmation and discovery of unexpected variants | Rapid genotyping of known SNPs |
| Application context | Variant validation and sequence-level confirmation | Large-scale known-SNP genotyping and epidemiological studies |
We therefore established a TaqMan qPCR assay for rs6923761 using buccal swab-derived DNA and compared the resulting genotype calls with Sanger sequencing in a preliminary cohort of adolescents. The study was designed to evaluate genotyping concordance and workflow feasibility; it was not designed to test associations with obesity, diabetes, or response to GLP-1RAs.
Methods
Study Participants
Twenty-two adolescent volunteers (11 male and 11 female; 12-18 years of age) were recruited through a school-based research activity. Buccal swab samples from all participants were used for rs6923761 genotyping. Exclusion criteria were self-reported diabetes, major chronic disease, acute oral inflammation, and antibiotic use within the previous 2 weeks. These criteria were used to avoid acute illness or oral conditions that could interfere with sample collection or DNA quality.
Ethics Approval and Informed Consent
The protocol was approved by the Institutional Ethics Committee of Beijing Zhenguo Integrative Chinese and Western Medicine Hospital and was conducted in accordance with the Declaration of Helsinki. Because all participants were minors, written informed consent was obtained from a legal guardian and assent was obtained from each participant before sampling. Samples and data were anonymized before laboratory analysis. Genotyping was performed for research purposes only and was not used to guide treatment.
DNA Extraction and Quality Control
Participants rinsed their mouths with water and refrained from eating or drinking for 30 min before sampling. Buccal mucosa from both cheeks was swabbed for approximately 30 s per side using disposable medical swabs20. Swab heads were immediately placed into 2-mL tubes containing DNA preservation solution (Swab DNA Storage Tube, catalog No. WE0400, Baiao Leibo Technology Co., Ltd.) and transported to the laboratory at room temperature within 48 h.
Genomic DNA was extracted with the MagPure Swab DNA KF Kit (catalog No. D6317-01, Huayunbio) on a KingFisher Flex automated magnetic-bead platform (Thermo Fisher Scientific, Waltham, MA, USA). The workflow included lysis, Proteinase K digestion, magnetic-bead capture, and ethanol-based washing. DNA concentration and A260/A280 and A260/A230 ratios were measured before PCR. All 22 DNA extracts provided sufficient material for both genotyping methods.
TaqMan qPCR Genotyping
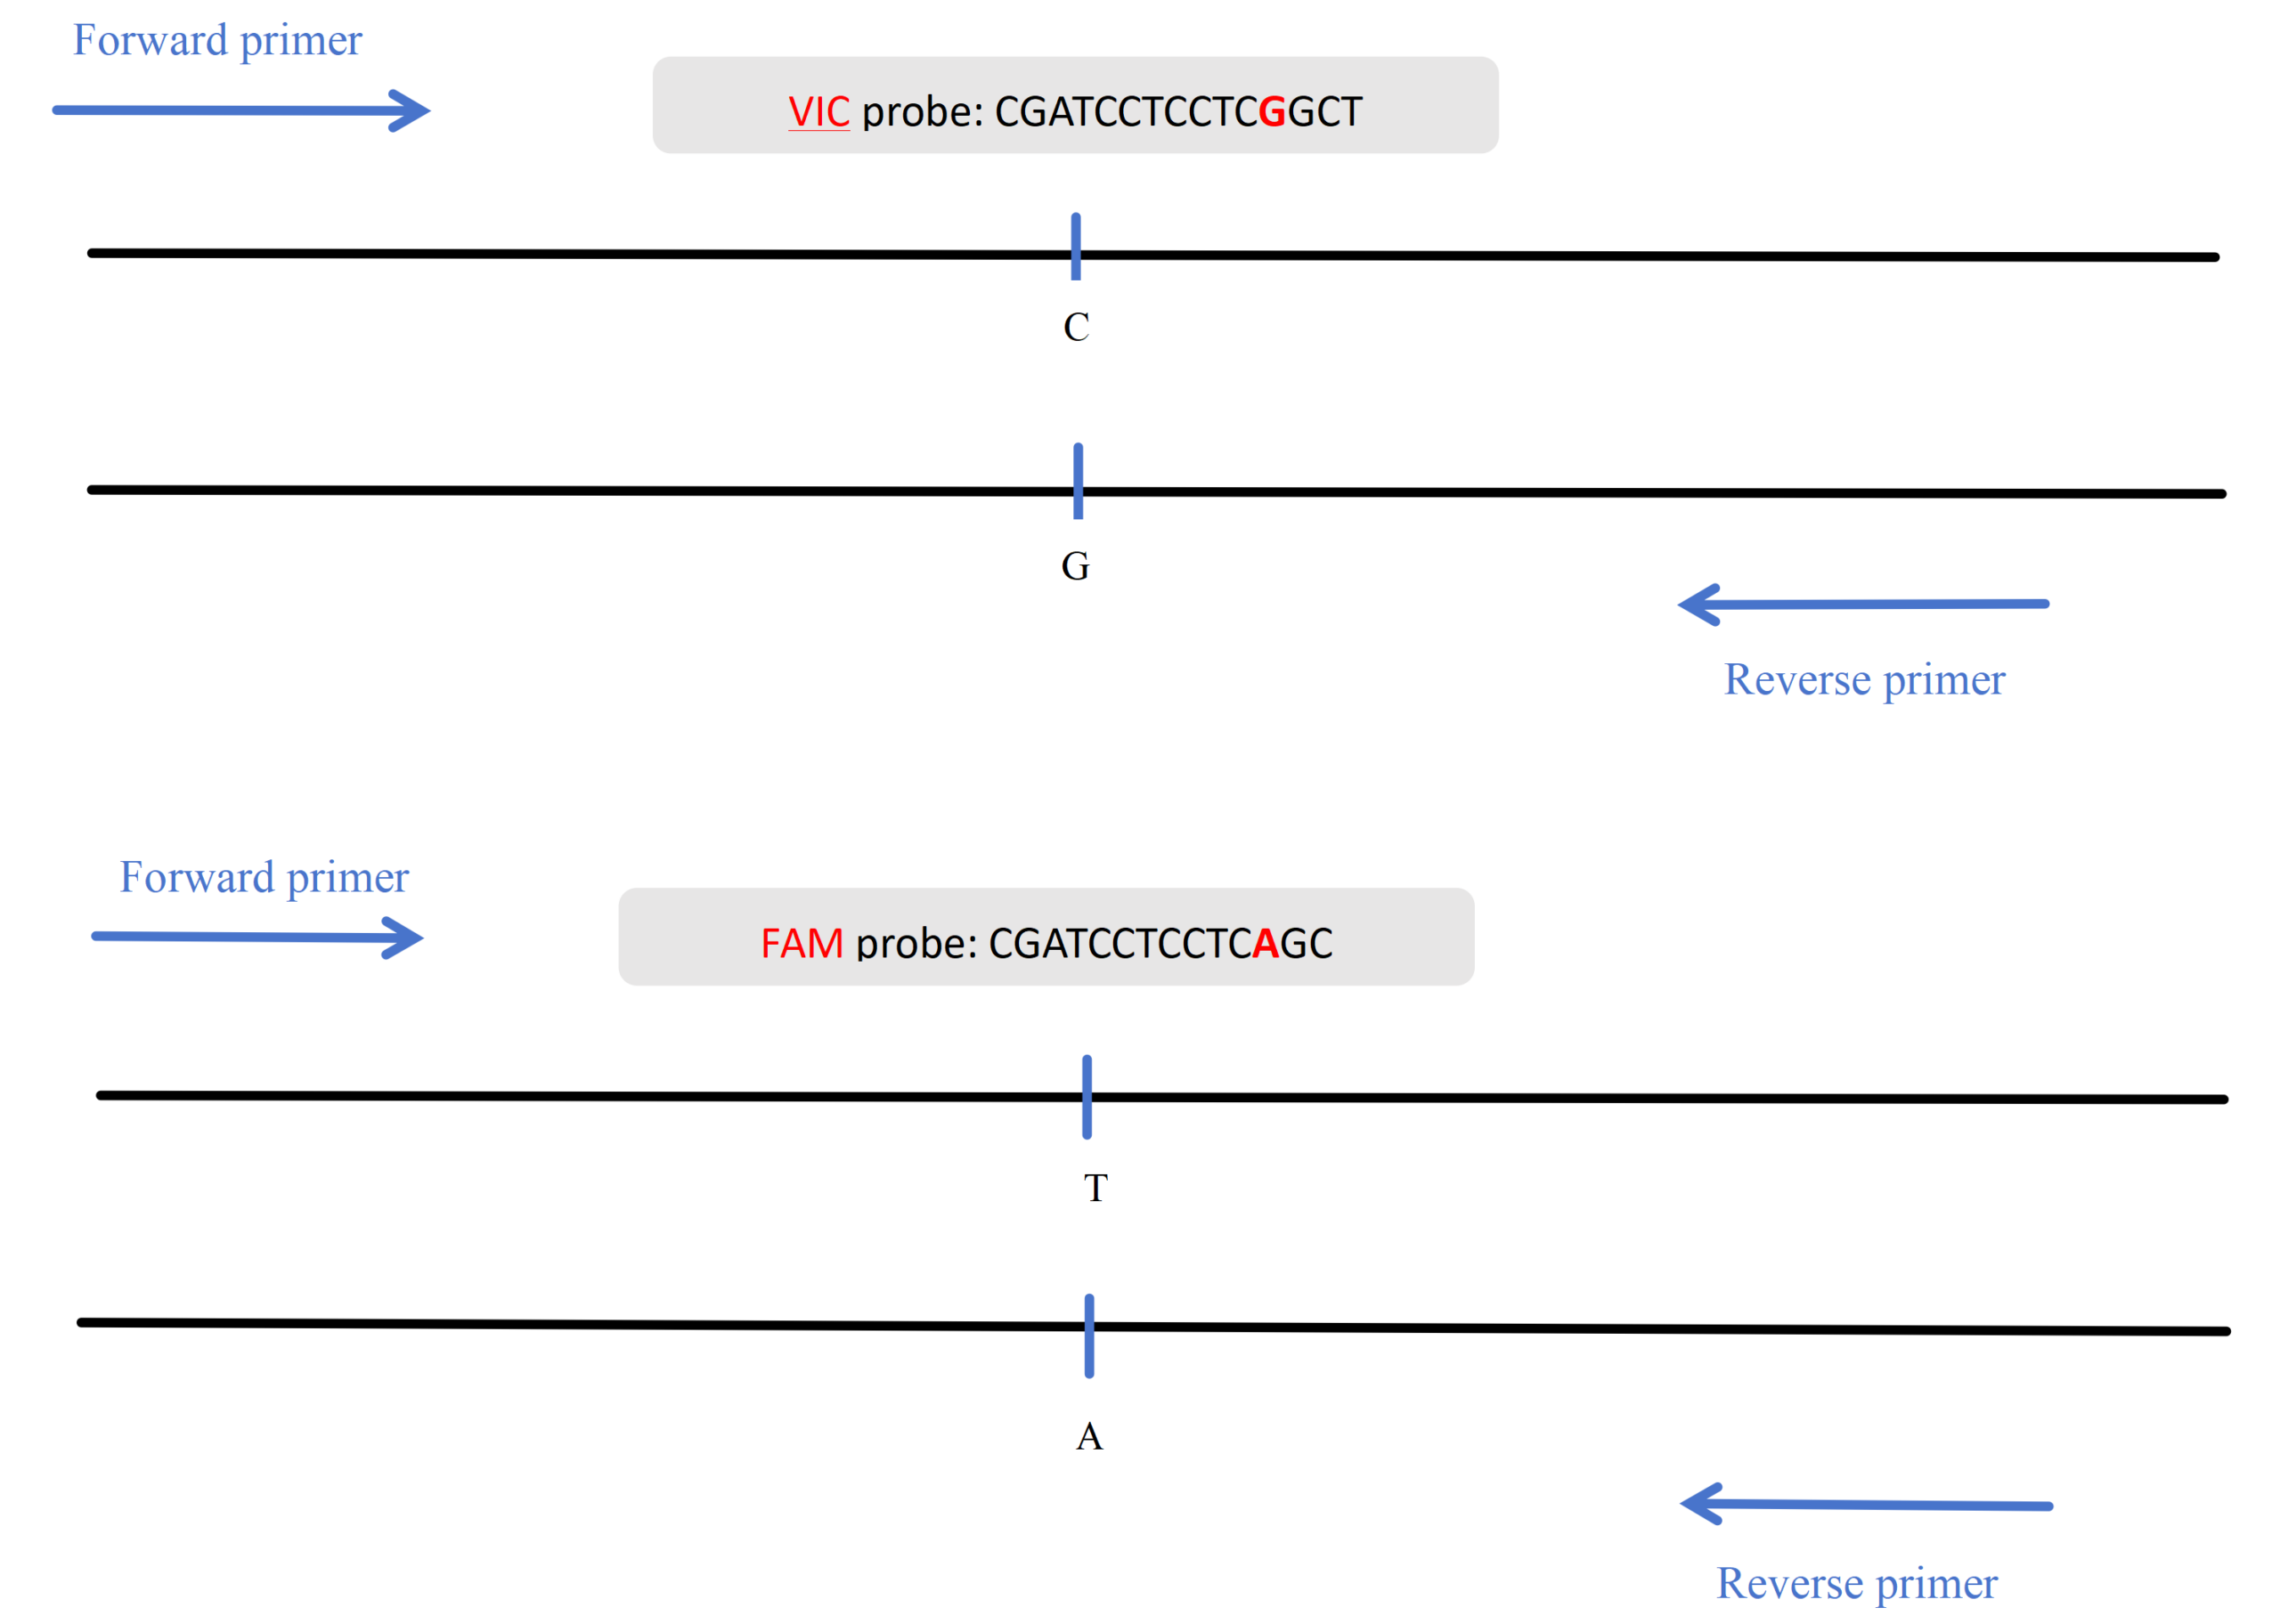
TaqMan qPCR was performed in accordance with the relevant MIQE reporting principles21. Reactions used Hieff Unicon Universal TaqMan Probe U+ qPCR Mix (Yeasen Biotechnology, Shanghai, China; catalog No. 16710ES60). Primers and probes were designed from the genomic sequence flanking rs6923761 and checked for specificity with Primer-BLAST before synthesis by Generay Biotechnology. The G-allele probe was labeled with VIC and the A-allele probe with 6-FAM; both probes carried a 3′ MGB non-fluorescent quencher. Final concentrations were 400 nM for each primer and 200 nM for each probe.
| Name | Sequence (5-prime to 3-prime) | Modification |
| rs6923761-Forward | CTCCTTCTCTGCTCTGGTTATCG | None |
| rs6923761-Reverse | GTCCGGGCCACCTTACCT | None |
| rs6923761-probe-G | CGATCCTCCTCGGCT | 5’ VIC, 3’ MGB/NFQ |
| rs6923761-probe-A | CGATCCTCCTCAGC | 5’ 6-FAM, 3’ MGB/NFQ |
| Component | qPCR volume (μL) | Final concentration | Sanger PCR volume (μL) |
| 2x qPCR or PCR master mix | 5 | 1x | 25 |
| Forward primer | 0.4 | 400 nM | 2 |
| Reverse primer | 0.4 | 400 nM | 2 |
| G probe | 0.2 | 200 nM | / |
| A probe | 0.2 | 200 nM | / |
| Sample DNA | 1 | Approximately 10-100 ng input | 1 |
| Nuclease-free water | 2.8 | / | 20 |
| Total | 10 | / | 50 |
| Step | Temperature | Time | Cycles |
| Initial background fluorescence collection | 60 ℃ | 30 sec | 1 |
| Pre-denaturation | 95 ℃ | 10 min | 1 |
| Denaturation | 95 ℃ | 15 sec | 40* |
| Annealing/extension and fluorescence detection | 60 ℃ | 1 min | |
| Final fluorescence collection | 60 ℃ | 30 sec | 1 |
* Fluorescence collection, detection channels: FAM, VIC
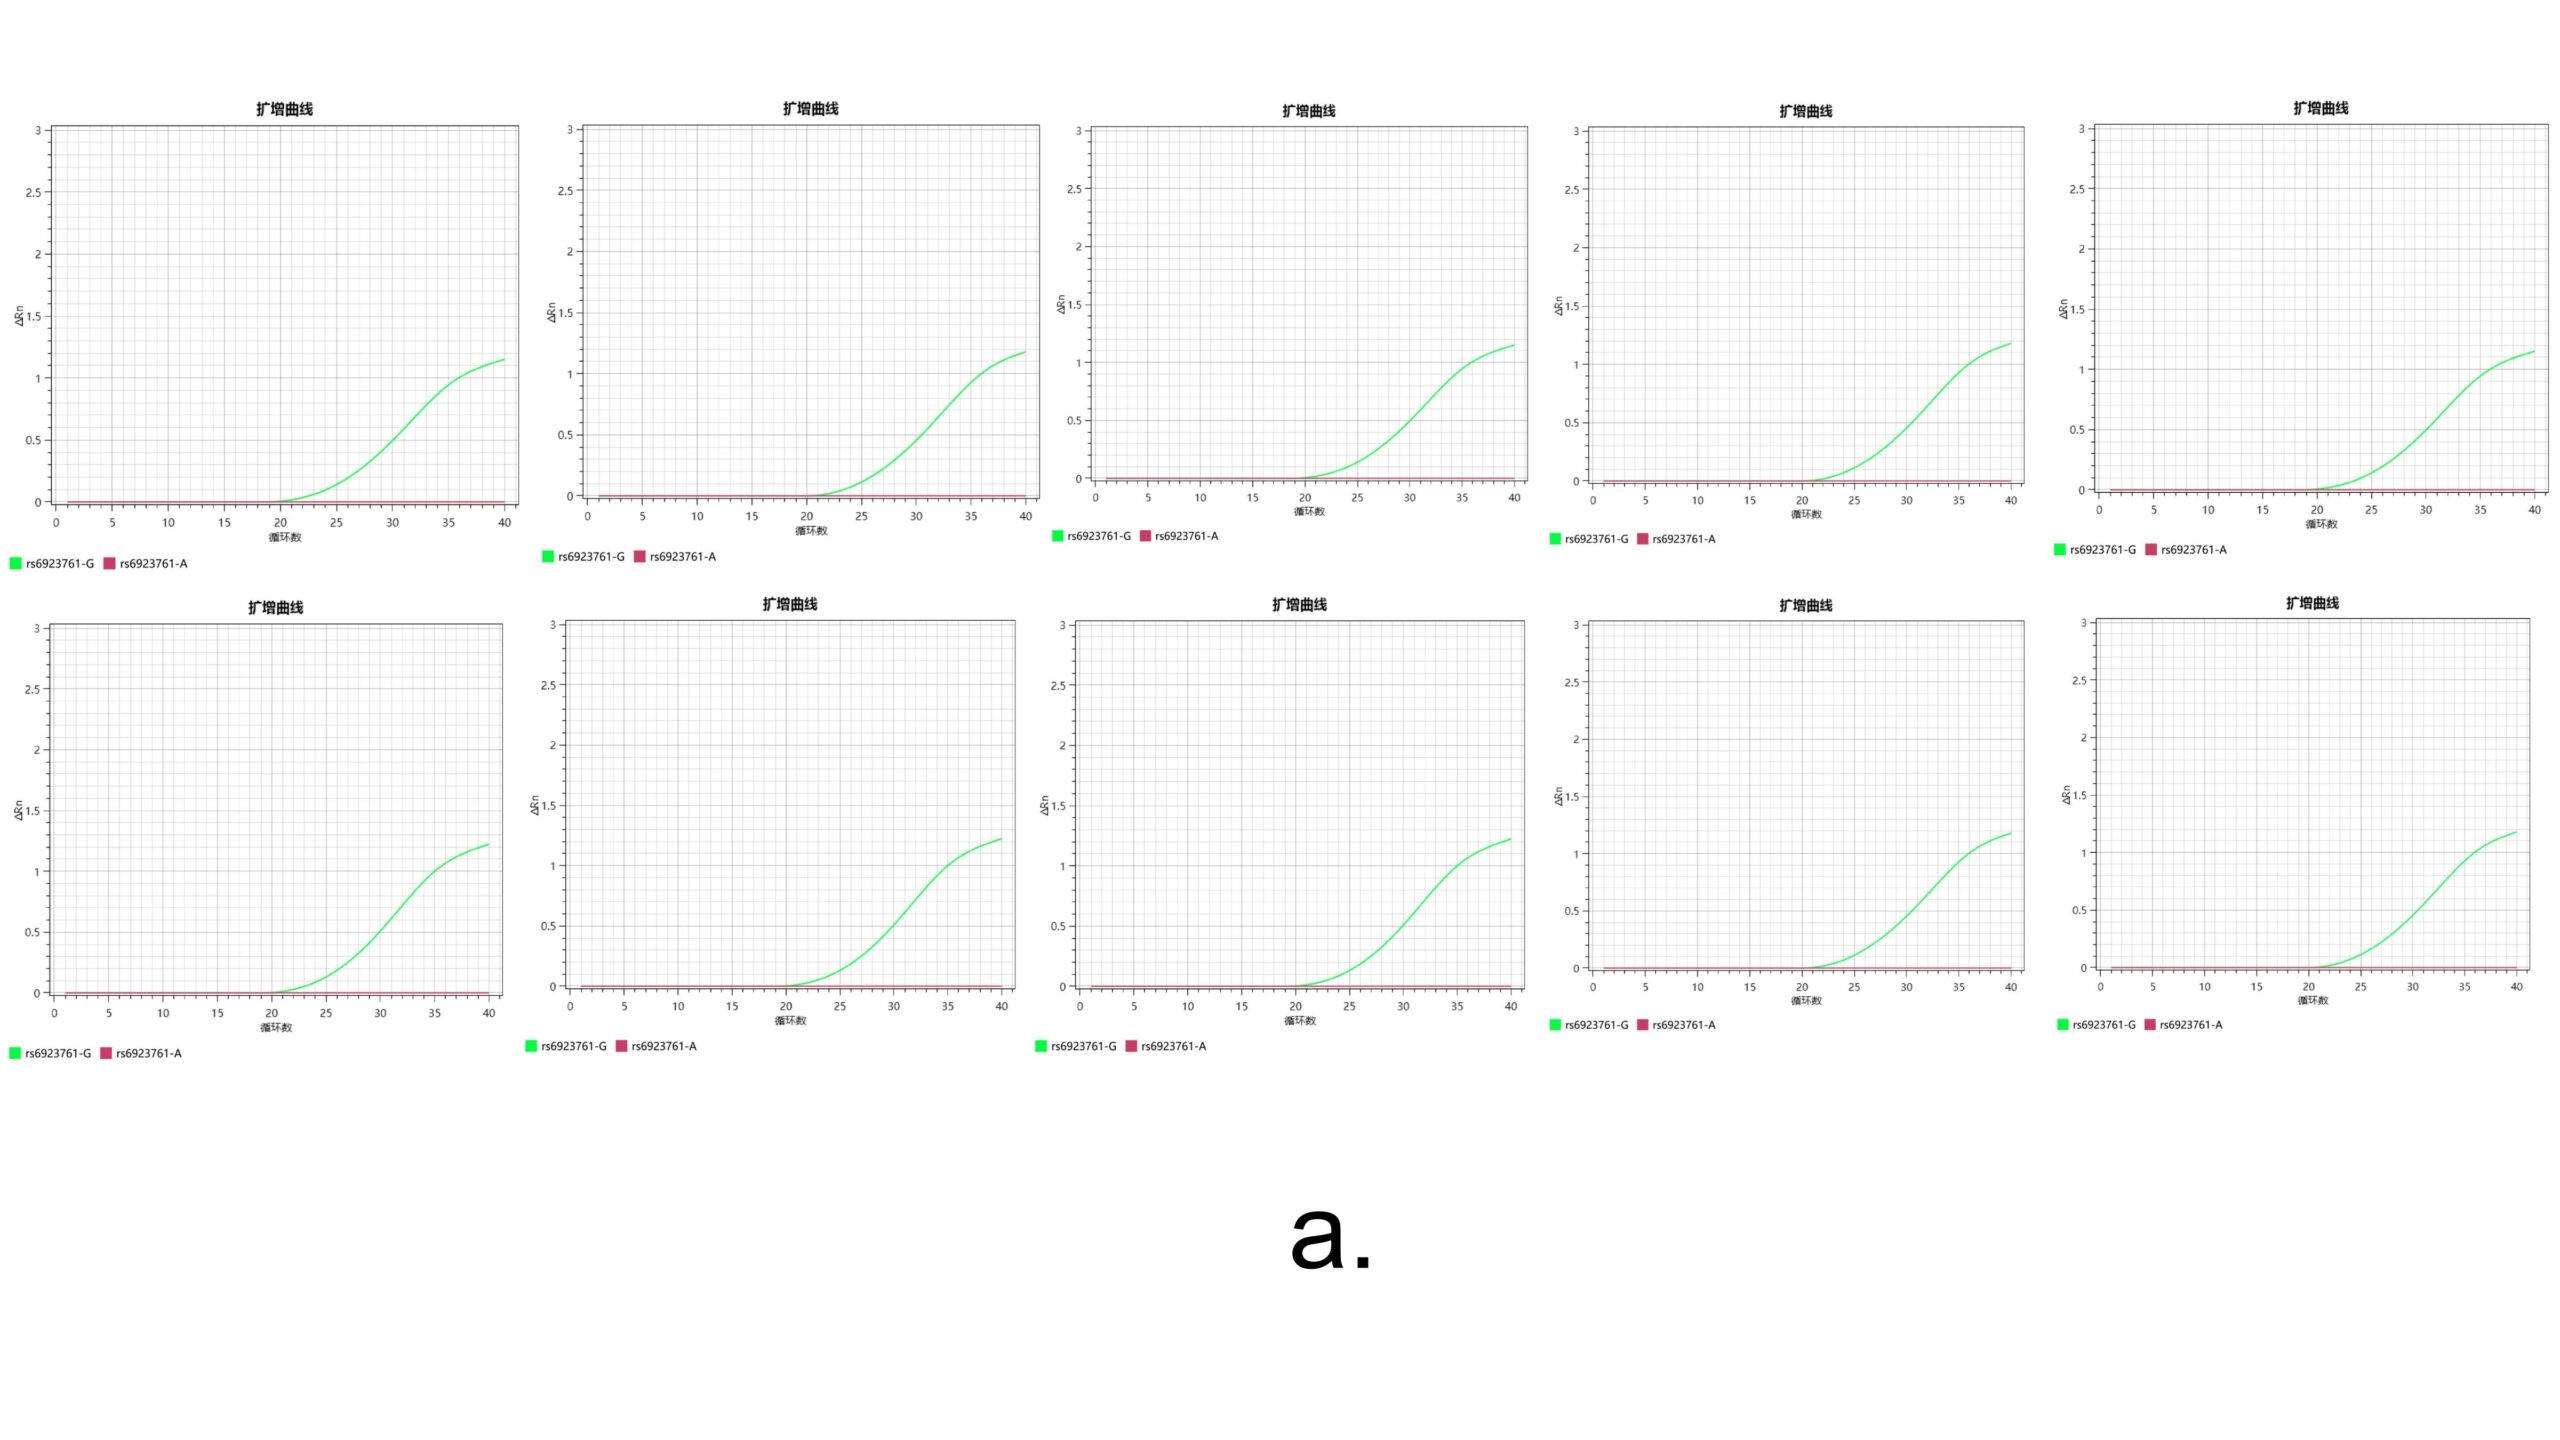
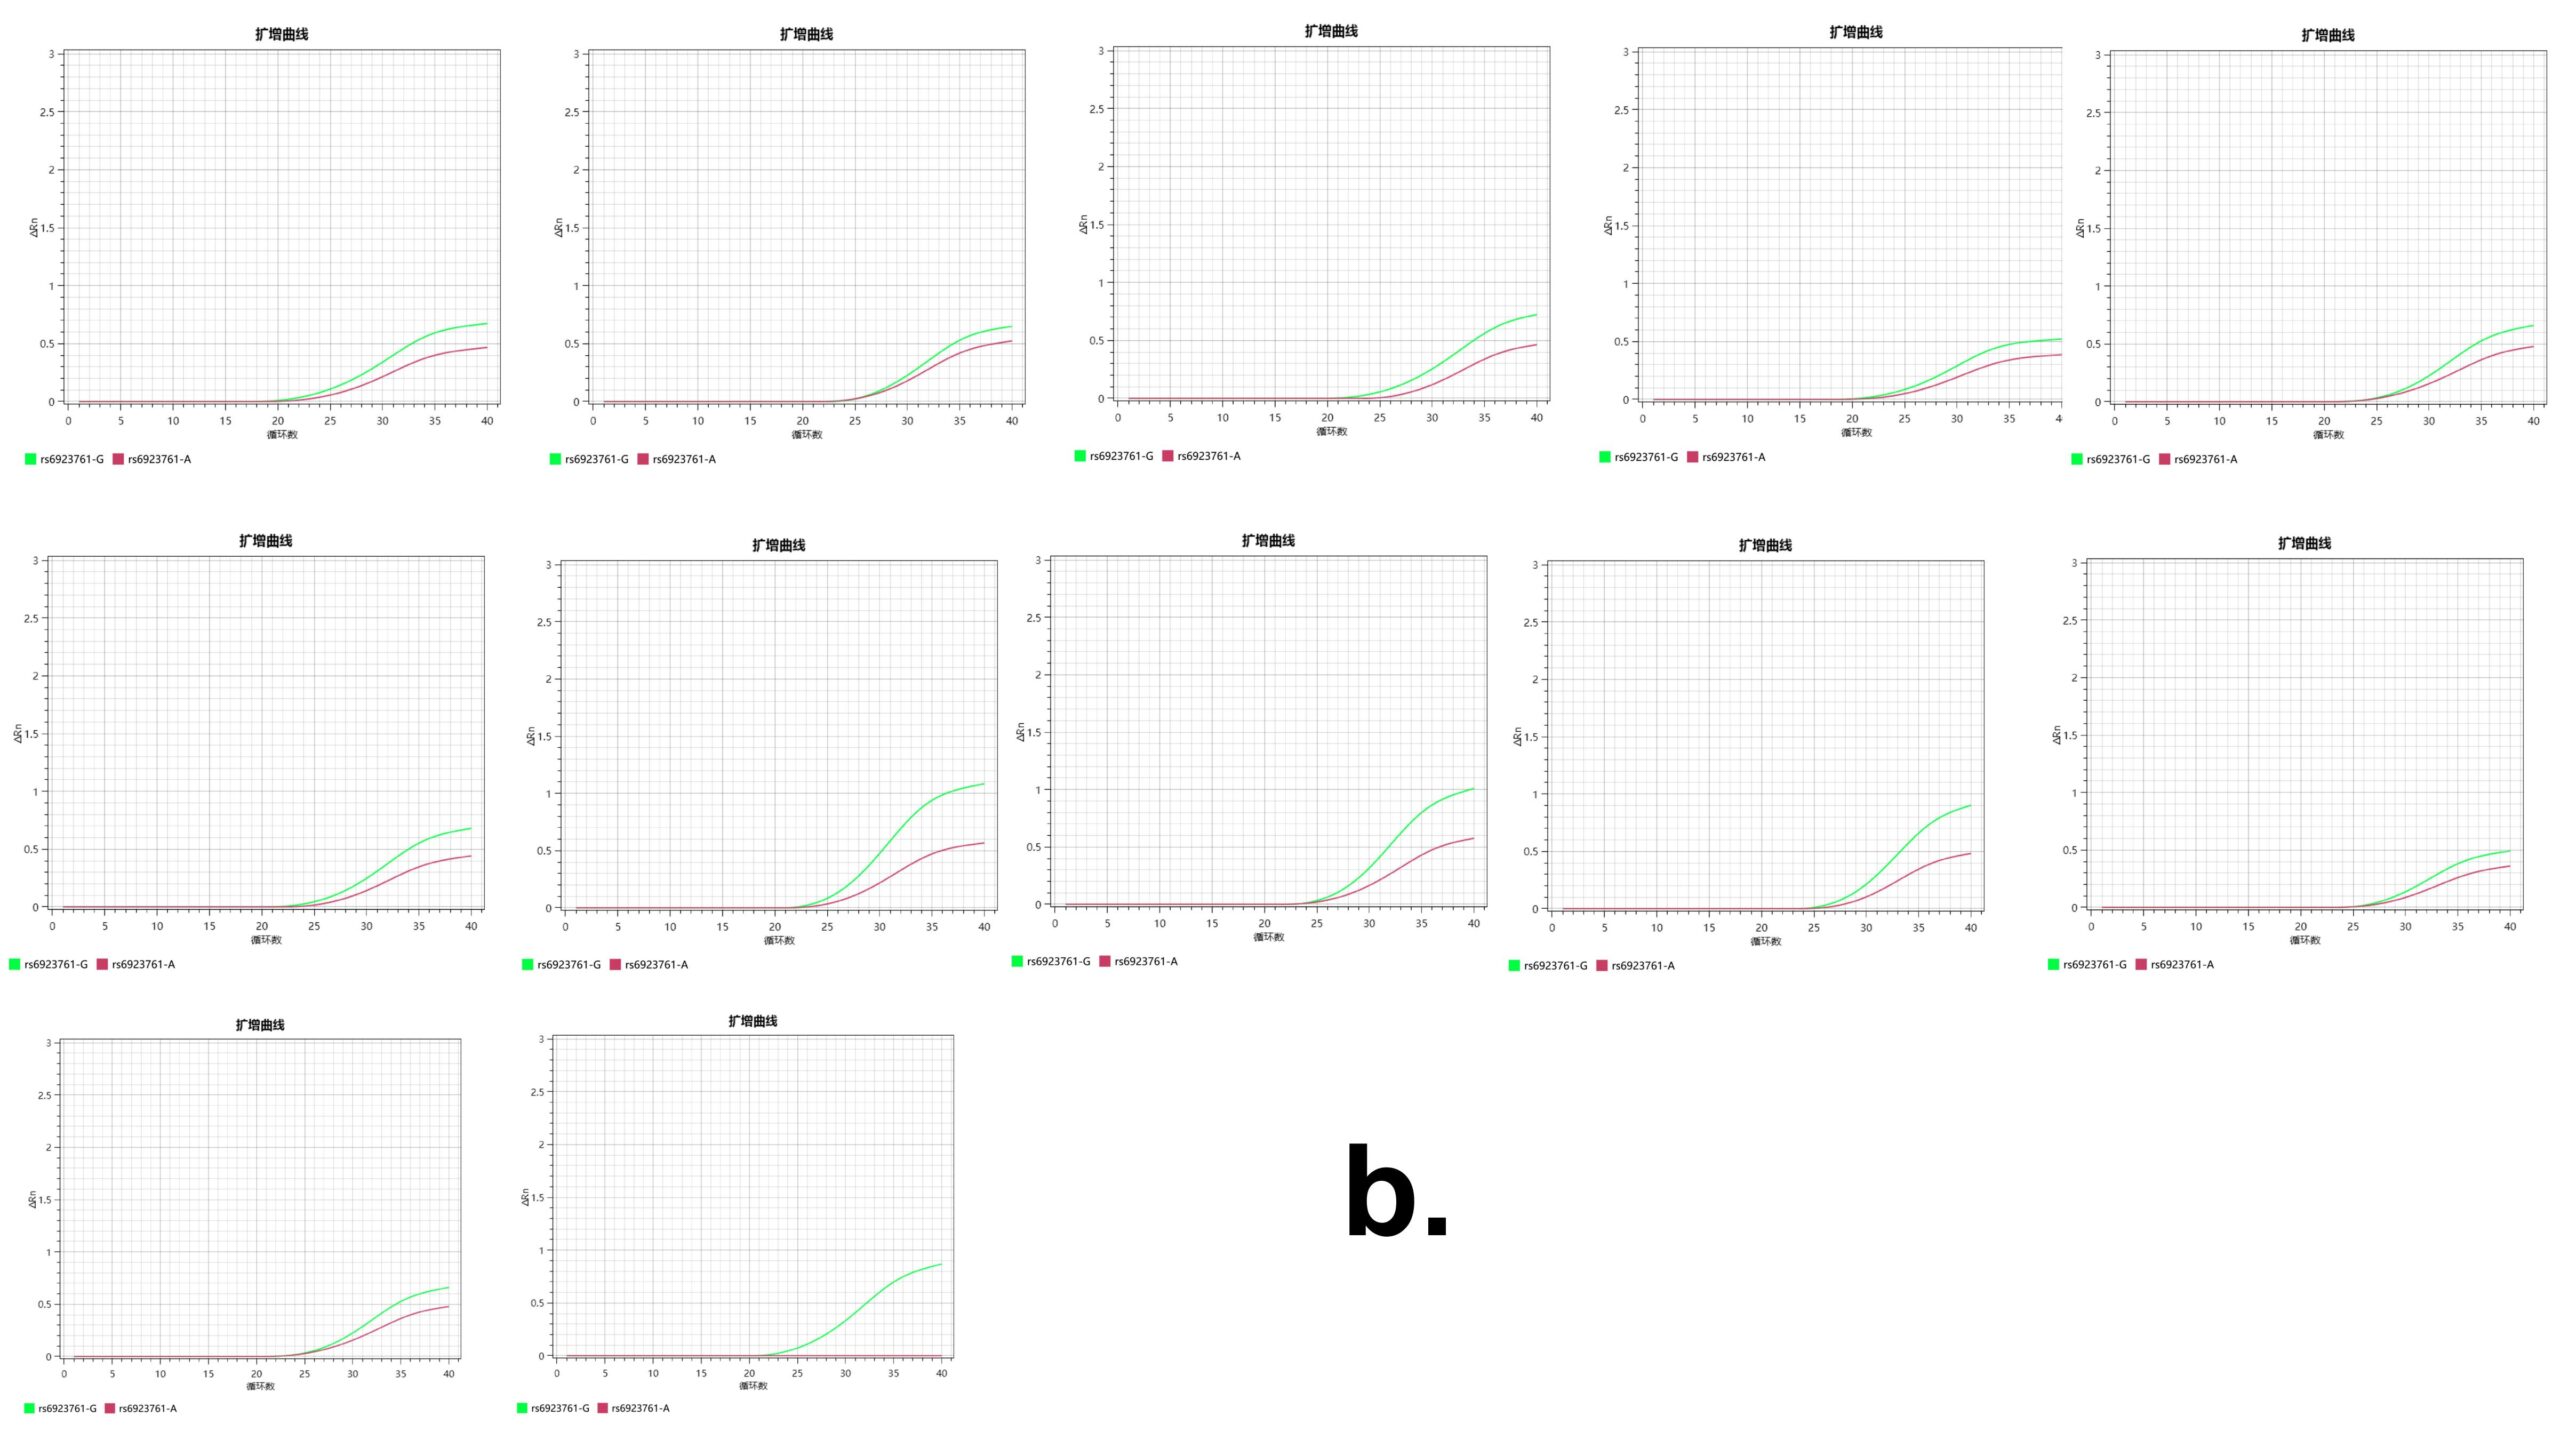
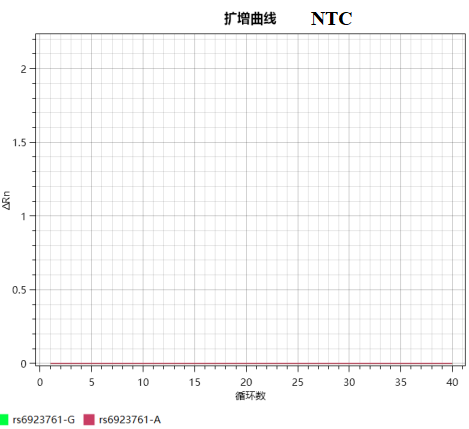
Each run included a no-template control (NTC) containing nuclease-free water. Amplification and endpoint fluorescence measurements were performed on an Archimed 384 high-throughput real-time PCR system (Kunpeng Gene), and genotype calls were generated with Archimed Analyzer software. Allelic discrimination was based on endpoint FAM/VIC clustering: VIC-only signal was called GG, FAM-only signal AA, and combined FAM/VIC signal GA. Samples without a clear cluster or with discordant replicate results were repeated.

Sanger Sequencing
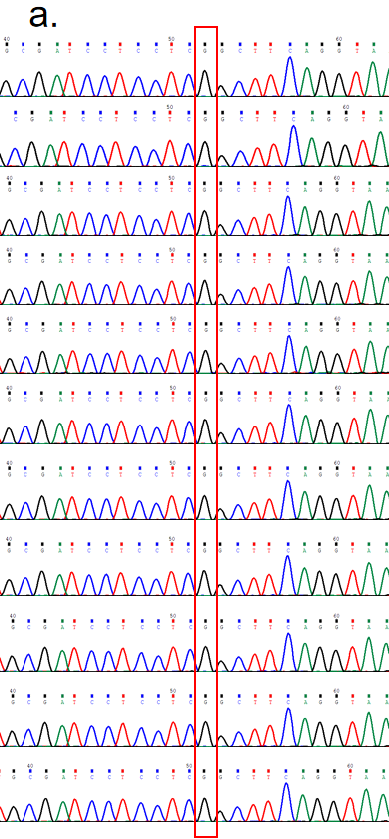
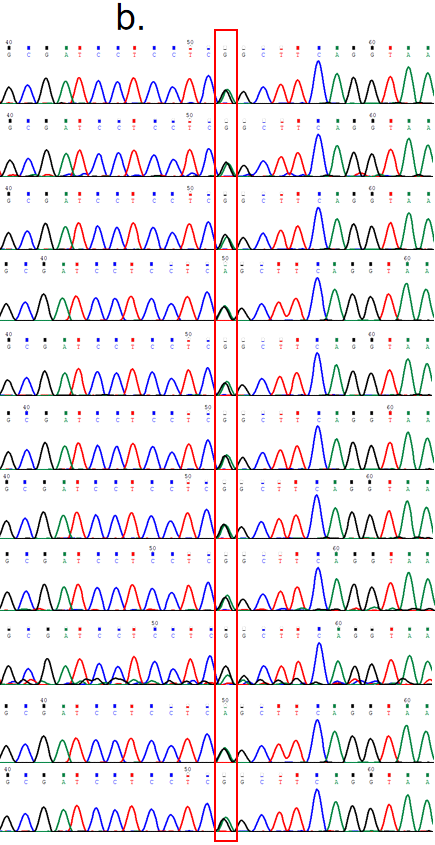
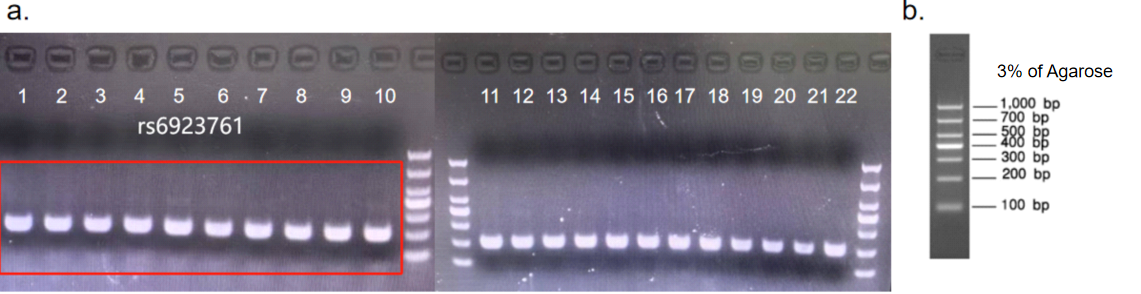
The region containing rs6923761 was amplified using the Sanger PCR reaction mixture shown in Table 3. The expected product was 214 bp, and amplification products were examined by agarose gel electrophoresis before sequencing. Sanger sequencing was performed on an ABI-3000-Px platform according to the laboratory protocol. Chromatograms were inspected at rs6923761: a single G peak was called GG, overlapping G/A peaks GA, and a single A peak AA. Samples with high background or ambiguous base calls were re-amplified and re-sequenced. The amplification primers were 5′-GCTACGCACTCTCCTTCTC-3′ (forward) and 5′-CAACCTCATATTCTACGGTCAG-3′ (reverse).
Statistical Analysis
Genotype counts and allele frequencies were calculated by direct counting. HWE was assessed by the chi-square test23. Concordance was defined as the proportion of samples with identical TaqMan qPCR and Sanger genotype calls. An exact binomial (Clopper-Pearson) 95% CI was calculated for the concordance rate24, and Cohen’s kappa was used to assess agreement beyond chance25. A two-sided p value <0.05 was considered statistically significant.
Results
DNA Yield and Purity
All 22 buccal swab samples yielded DNA that could be analyzed by both methods. DNA concentrations ranged from 18.6 to 76.4 ng/μL (mean, 42.8 ng/μL). A260/A280 ratios ranged from 1.78 to 1.93 and A260/A230 ratios from 1.86 to 2.21 (Table 5). No sample was excluded because of insufficient DNA yield or purity.
Table 5 | DNA concentration and purity of the 22 oral swab samples.
| Sample ID | DNA concentration (ng/μL) | A260/A280 | A260/A230 |
| 1 | 35.2 | 1.84 | 2.03 |
| 2 | 41.7 | 1.86 | 2.08 |
| 3 | 28.9 | 1.81 | 1.96 |
| 4 | 52.4 | 1.89 | 2.12 |
| 5 | 46.8 | 1.87 | 2.05 |
| 6 | 31.5 | 1.82 | 1.91 |
| 7 | 58.6 | 1.90 | 2.16 |
| 8 | 33.7 | 1.79 | 1.88 |
| 9 | 39.4 | 1.85 | 2.01 |
| 10 | 44.1 | 1.88 | 2.09 |
| 11 | 63.2 | 1.91 | 2.18 |
| 12 | 38.6 | 1.78 | 1.86 |
| 13 | 37.9 | 1.84 | 2.00 |
| 14 | 49.5 | 1.87 | 2.07 |
| 15 | 55.3 | 1.90 | 2.15 |
| 16 | 33.8 | 1.83 | 1.94 |
| 17 | 72.1 | 1.92 | 2.20 |
| 18 | 26.4 | 1.80 | 1.89 |
| 19 | 47.6 | 1.86 | 2.06 |
| 20 | 76.4 | 1.93 | 2.21 |
| 21 | 40.3 | 1.85 | 2.02 |
| 22 | 60.7 | 1.91 | 2.17 |
Genotyping by TaqMan qPCR
Endpoint fluorescence separated the samples into two genotype clusters. Eleven samples showed predominantly VIC fluorescence and were called GG, while 11 showed both VIC and FAM signals and were called GA. No FAM-only AA cluster was observed. The NTC remained outside the genotype clusters and showed no detectable allele-specific signal (Figure 3). The resulting genotype frequencies were 50.0% GG, 50.0% GA, and 0% AA; the G and A allele frequencies were 75.0% and 25.0%, respectively.
| Genotype | TaqMan-qPCR (n) | Sanger sequencing (n) |
| GG | 11 | 11 |
| GA | 11 | 11 |
| AA | 0 | 0 |
| Total | 22 | 22 |
The observed genotype distribution did not differ significantly from HWE (expected counts: GG, 12.38; GA, 8.25; AA, 1.38; chi-square = 2.44, p = 0.118). TaqMan qPCR and Sanger sequencing agreed in all 22 samples, giving a concordance rate of 100% (22/22; exact 95% CI, 84.6%-100%) and a Cohen’s kappa of 1.00.
Concordance with Sanger Sequencing
Sanger sequencing confirmed the same 11 GG and 11 GA genotypes identified by TaqMan qPCR. GG samples showed a single G peak at rs6923761, whereas GA samples showed overlapping G and A peaks (Figure 4). One sample had substantial background in the initial sequencing run; repeat amplification and sequencing produced an interpretable chromatogram and confirmed the GA genotype. No discordant genotype call was observed between the two methods.
Discussion
Assay Performance and Concordance
The main finding of this study is the complete agreement between TaqMan qPCR and Sanger sequencing for the 22 samples tested. The two methods assigned the same 11 samples as GG and the same 11 as GA, and the qPCR NTC remained negative. For a known biallelic SNP, the TaqMan workflow has a practical advantage because amplification and genotype discrimination are completed in a closed tube without a separate sequencing step. The present data support the feasibility of the assay for rs6923761 genotyping, but they should not be interpreted as a complete analytical validation.
Interpretation of rs6923761 and Study Scope
The A-allele frequency in this small cohort was 25.0%, and no AA homozygote was observed. Given the sample size, the absence of an AA sample limits the direct evidence for the FAM-only genotype cluster and is more important for assay validation than the observed HWE result. The rs6923761 variant has been associated in previous studies with metabolic phenotypes and with responses to GLP-1RAs, but the direction and magnitude of these associations have not been consistent across studies26. Because no obesity phenotype, glycemic measurements, or treatment-response data were collected here, the present study cannot address the clinical relevance of the variant.
Limitations
Several limitations should be considered. First, the cohort was small, and the exact 95% CI around the observed 100% concordance extended down to 84.6%. Second, no AA homozygous sample was available, so all three possible genotype classes were not directly verified. Third, the study did not include serial template dilution, intra- and inter-run reproducibility testing, robustness experiments, or a formal limit-of-detection analysis. The small expected AA count also limits the usefulness of a chi-square HWE test in this cohort. Finally, participants were recruited from a single school-based population, and the genotype frequencies should not be generalized to the broader adolescent population. Future validation should include confirmed AA-positive material, replicate testing across runs, and a larger independent sample set.
Conclusion
A TaqMan qPCR assay for GLP1R rs6923761 produced the same genotype calls as Sanger sequencing in 22 buccal swab samples containing GG and GA genotypes. The assay provides a rapid closed-tube approach for genotyping this known SNP. Validation with confirmed AA samples and formal analytical performance testing is still required before the method is used for clinical interpretation or pharmacogenetic decision-making.
Acknowledgements
I am grateful to Hongyang Liu and Youyuan Cao for their support and encouragement throughout this project. I would also like to thank Yayuan Jiang for her guidance and valuable feedback throughout the process of this study.
References
- X. F. Pan, L. Wang, A. Pan. Epidemiology and determinants of obesity in China. Lancet Diabetes & Endocrinology 9, 373–392 (2021). [↩]
- C. Y. Ji, T. J. Chen. Empirical changes in the prevalence of overweight and obesity among Chinese students from 1985 to 2010 and corresponding preventive strategies. Biomedical and Environmental Sciences 26, 1–12 (2013). [↩]
- G. Twig, I. Zucker, A. Afek, T. Cukierman-Yaffe, C.D. Bendor, E. Derazne, M. Lutski, T. Shohat, O. Mosenzon, D. Pinhas-Hamiel, S. Tiosano, I. Raz, H. Gerstein, A. Tirosh. Adolescent obesity and early-onset type 2 diabetes. Diabetes Care 43, 1487–1495 (2020). [↩]
- D. J. Magliano, E. J. Boyko, IDF Diabetes Atlas 10th edition scientific committee. *IDF diabetes atlas*. 10th ed. Brussels: International Diabetes Federation (2021). [↩]
- D. A. De Luis, R. Aller, O. Izaola, R. Bachiller. Role of rs6923761 gene variant in glucagon-like peptide 1 receptor in basal GLP-1 levels, cardiovascular risk factor and serum adipokine levels in naive type 2 diabetic patients. Journal of Endocrinological Investigation 38, 143–147 (2015). [↩]
- S. ‘ajan, L. M. Dickson, E. Mathew, C. M. Orr, J. H. Ellenbroek, L. H. Philipson, B. Wicksteed. Chronic hyperglycemia downregulates GLP-1 receptor signaling in pancreatic beta-cells via protein kinase A. Molecular Metabolism 4, 265–276 (2015). [↩]
- UniProt Consortium. UniProt: the universal protein knowledgebase. Nucleic Acids Research 51, D523–D531 (2023). [↩]
- C. Liu, X. Bao, Y. Tian, P. Xue, Y. Wang, Y. Li. Polymorphisms in the glucagon-like peptide-1 receptor gene and their interactions on the risk of osteoporosis in postmenopausal Chinese women. PLOS ONE 18, e0295451 (2023). [↩] [↩]
- D. A. de Luis, M. Ballesteros, A. L. Guzman, E. Ruiz, C.Muñoz, M.A. Penacho, P. Iglesias, A. Maldonado, V. Puigdevall, M. Delgado. rs6923761 gene variant in glucagon-like peptide receptor: allelic frequencies and influence on cardiovascular risk factors in a multicenter study of Castilla-Leon. Clinical Nutrition 37, 2144–2148 (2018). [↩] [↩]
- V. Chedid, P. Vijayvargiya, P. Carlson, K. Van Malderen, A. Acosta, A. Zinsmeister, M. Camilleri. Allelic variant in the glucagon-like peptide 1 receptor gene associated with greater effect of liraglutide and exenatide on gastric emptying: a pilot pharmacogenetics study. Neurogastroenterology and Motility 30, e13313 (2018). [↩] [↩]
- M. Yu, K. Wang, H. Liu, R. Cao. GLP1R variant is associated with response to exenatide in overweight Chinese type 2 diabetes patients. Pharmacogenomics 20, 273–277 (2019). [↩] [↩]
- P. Luo, Y. Fan, Y. Xiong, H. Feng, Z. Yang, C. Zhang, B. Mei. Genetic variants of the GLP-1R gene affect the susceptibility and glucose metabolism of gestational diabetes mellitus: a two-center nested case-control study. Diabetology & Metabolic Syndrome 14, 190 (2022). [↩] [↩]
- A. Y. Dawed, A. Mari, A. Brown, T. J. McDonald, L. Li, S. Wang. Pharmacogenomics of GLP-1 receptor agonists: a genome-wide analysis of observational data and large randomised controlled trials. Lancet Diabetes & Endocrinology 11, 33–41 (2023). [↩] [↩]
- M. Mashayekhi, B. I. Safa, H. Nian, J. K. Devin, J. L. Gamboa, C. Yu, R. Chen, J. A. Beckman, J. R. Koethe, H. J. Silver, K. Niswender, J. M. Luther, N. J. Brown. Rising stars: effects of a GLP-1 receptor polymorphism on responses to liraglutide. Journal of Endocrinology 267, e250174 (2025). [↩] [↩]
- E. Kamau, S. Alemayehu, K. C. Feghali, L. S. Tolbert, B. Ogutu, C. F. Ockenhouse. Development of a TaqMan allelic discrimination assay for detection of single nucleotides polymorphisms responsible for anti-malarial drug resistance. Malaria Journal 11, 23 (2012). [↩]
- K. J. Livak, S. J. Flood, J. Marmaro, W. Giusti, K. Deetz. Oligonucleotides with fluorescent dyes at opposite ends provide a quenched probe system useful for detecting PCR product and nucleic acid hybridization. PCR Methods and Applications 4, 357–362 (1995). [↩]
- C. Broccanello, C. Chiodi, A. Funk, J. M. McGrath, L. Panella, P. Stevanato. Comparison of three PCR-based assays for SNP genotyping in plants. Plant Methods 14, 28 (2018). [↩]
- R. Osaki, H. Imaeda, H. Ban, T. Aomatsu, S. Bamba, T. Tsujikawa, M. Sasaki, Y. Fujiyama, A. Andoh. Accuracy of genotyping using the TaqMan PCR assay for single nucleotide polymorphisms responsible for thiopurine sensitivity in Japanese patients with inflammatory bowel disease. Experimental and Therapeutic Medicine 2, 783–786 (2011). [↩]
- K. Muneeswaran, V. A. de Silva, U. Branavan, M. Dayabandara, R. Hanwella, N. V. Chandrasekharan. PCR-based SNP genotyping: a comprehensive comparison of methods for affordable and accurate detection of class IV mutations. Analytica Chimica Acta 1354, 343994 (2025). [↩]
- C. Theda, S. H. Hwang, A. Czajko, Y.J. Loke, P. Leong, J. M.Craig. Quantitation of the cellular content of saliva and buccal swab samples. Scientific Reports 8, 6944 (2018). [↩]
- S. A. Bustin, V. Benes, J. A. Garson, J. Hellemans, J. Huggett, M. Kubista, R. Mueller, T. Nolan, M. W. Pfaffl, G. L. Shipley, J. Vandesompele, C. T. Wittwer. The MIQE guidelines: minimum information for publication of quantitative real-time PCR experiments. Clinical Chemistry 55, 611–622 (2009). [↩]
- Jia X, Zhang L, Li Q, Zeng Q, Hu J, Bao Z, Wang M. Development and a TaqMan probe-based qPCR assay for Vibrio parahaemolyticus causing translucent post-larvae disease (TPD) detection in Litopenaeus vannamei. Journal of Invertebrate Pathology 216, 108574 (2026). [↩]
- S. Rodriguez, T. R. Gaunt, I. N. M. Day. Hardy-Weinberg equilibrium testing of biological ascertainment for Mendelian randomization studies. American Journal of Epidemiology 169, 505–514 (2009). [↩]
- C. J. Clopper, E. S. Pearson. The use of confidence or fiducial limits illustrated in the case of the binomial. Biometrika 26, 404–413 (1934). [↩]
- D. Gobena, E. K. Gudina, T. T. Degfie, T. Girma, G. Gebre, A. Abdissa, F. G. Tafesse, T. Gelanew, Z. Mekonnen. Comparative evaluation of in-house ELISA and two commercial serological assays for the detection of antibodies against SARS-CoV-2. Scientific Reports 15, 13853 (2025). [↩]
- A. S. Kelly, S. C. Armstrong, M. P. Michalsky, C. K. Fox. Obesity in adolescents: a review. JAMA 322, 738–748 (2024). [↩]